Description
MOTS-c is a 16-residue peptide encoded in the mitochondrial 12S rRNA region. It contains two methionine residues and one tryptophan, all of which are oxidation sensitive, so vials should stay sealed and cold until immediately before use.
MOTS-c: what the published research shows
Compiled by NADA-Labs from the peer-reviewed literature cited below. No own study data.
MOTS-c (mitochondrial open reading frame of the 12S rRNA type-c) is a 16-amino-acid peptide encoded by a short open reading frame within the mitochondrial 12S rRNA gene and is classified as a mitochondrial-derived peptide. In cell and rodent studies it inhibits the folate cycle and de novo purine synthesis, leading to AICAR accumulation and AMPK activation, with skeletal muscle described as its main target tissue. The published research is concentrated on skeletal-muscle insulin sensitivity, diet-induced obesity, physical performance and age-related decline in mice, with additional rodent work on bone loss and cardiac function. Human data consist of observational studies of endogenous circulating MOTS-c (exercise, lipid infusion, endothelial dysfunction, an mtDNA variant); no peer-reviewed interventional human trial of exogenous MOTS-c was found in PubMed.
Evidence base: Predominantly mouse and rat models plus in vitro work; human evidence is limited to observational studies of endogenous MOTS-c levels (n = 10 to 27,527), including a 10-person exercise-response study in healthy young men. A substantial share of the foundational work comes from one group (USC, Lee/Cohen) with declared consulting and shareholder ties to CohBar, Inc.
Key studies at a glance
| Study | Model | Design | Main result |
|---|---|---|---|
| Lee 20151 | Mice (C57BL/6, CD-1), high-fat diet; L6/HEK293 cells | Vehicle-controlled, i.p., 7 days (clamp) and 8 weeks (diet), n = 6-10 | Clamp glucose infusion rate approx. +30 %; high-fat-diet weight gain and hyperinsulinaemia prevented; aged-muscle insulin response restored |
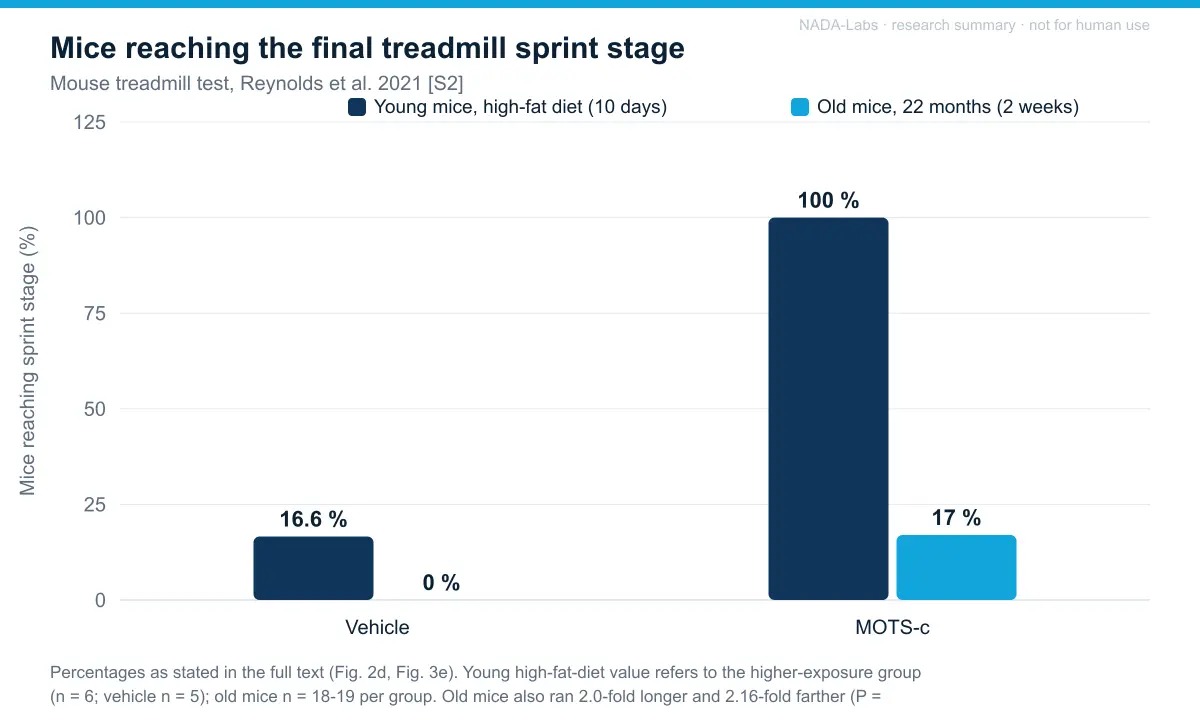
| Reynolds 20212 | Mice aged 2, 12, 22 months; C2C12 cells; 10 human exercise volunteers | Vehicle-controlled, i.p., 10-14 days; late-life intermittent treatment with lifelong follow-up, n = 5-19 | Old mice ran 2.0x longer, 2.16x farther; 17 % vs. 0 % reached sprint; grip strength and gait improved at >30 months; lifespan P = 0.23 (n.s.) |
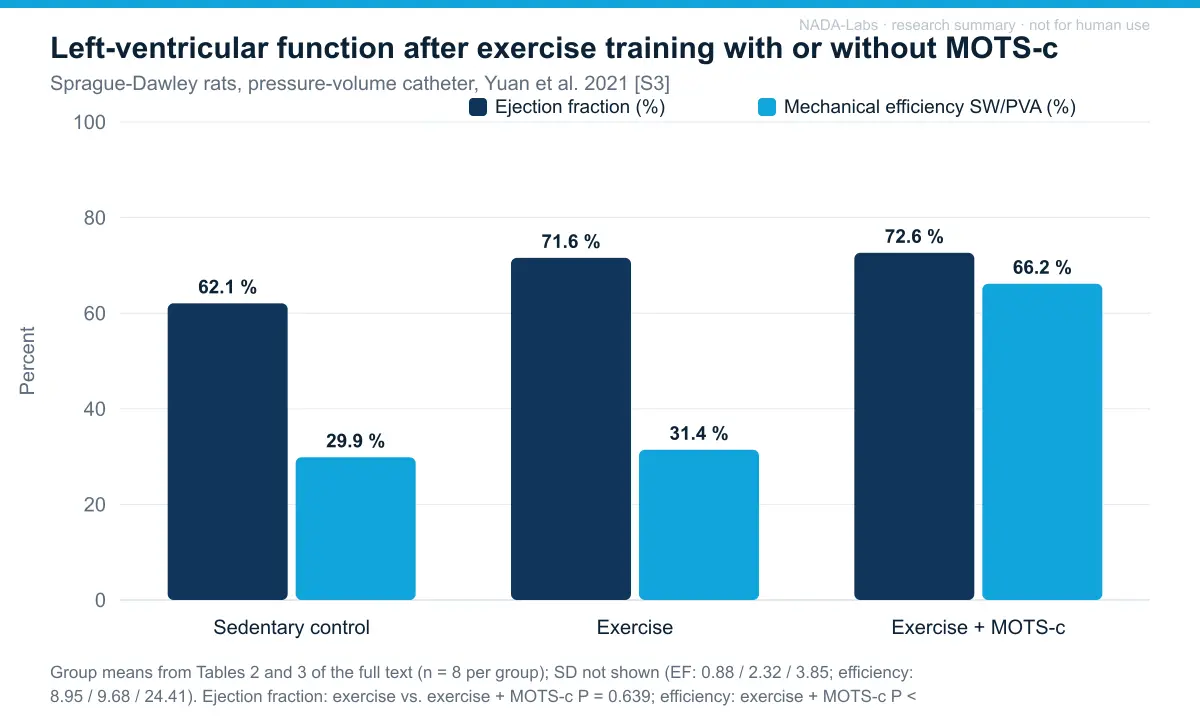
| Yuan 20213 | Sprague-Dawley rats, treadmill training | Three groups (control, exercise, exercise + MOTS-c), n = 8 each; P-V catheter | Mechanical efficiency 66 % vs. 31 % (exercise alone); PRSW slope 103 vs. 71; ejection fraction unchanged (72.6 vs. 71.6 %) |
| Zempo 20214 | Human cohorts (n = 27,527) plus high-fat-fed mice, both sexes | Meta-analysis of m.1382A>C carriers; water-controlled mouse study, 21 days, n = 8-12 | Male C-allele carriers: higher T2D prevalence; wild-type MOTS-c reduced weight and improved glucose tolerance in male but not female mice; K14Q variant less active |
| Ramanjaneya 20195 | Women with PCOS and healthy controls (endogenous MOTS-c) | Intralipid/saline infusion with clamp; repeated after 8 weeks of exercise | Lipid infusion raised plasma MOTS-c to 232 % (controls) and 349 % (PCOS) of basal; insulin blunted the rise; exercise training did not change circulating levels |
| Qin 20186 | Angina patients without coronary lesions (n = 40); rat aortic rings | Cross-sectional: normal endothelial function vs. dysfunction (20 each); organ chamber | Plasma MOTS-c lower with endothelial dysfunction (P = 0.007); correlates with coronary endothelial function; no direct vasoactivity |
| Ming 20167 | Ovariectomised mice; RANKL osteoclast assay | 12 weeks of injections; micro-CT | Bone loss significantly alleviated; osteoclast differentiation inhibited, partly AMPK-dependent |
Human data: endogenous MOTS-c (observational, no peptide administered)
| Study | Population / n | Measurement | Finding |
|---|---|---|---|
| Reynolds 20212 | 10 sedentary healthy young men (24.5 +/- 3.7 years) | Muscle biopsy and plasma before, during, after cycling | Muscle MOTS-c 11.9-fold after exercise; plasma 1.6-fold during, 1.5-fold after; baseline after 4 h rest |
| Ramanjaneya 20195 | Women with PCOS and healthy controls | Plasma ELISA during intralipid infusion and clamp | 232-349 % of basal with lipid; reduced to 165-183 % with insulin (P < 0.05 in PCOS) |
| Qin 20186 | 40 angina patients (20 with endothelial dysfunction) | Aortic plasma ELISA at catheterisation | Lower MOTS-c in endothelial dysfunction (P = 0.007); positive correlation with microvascular (P = 0.01) and epicardial (P = 0.02) function |
| Zempo 20214 | 27,527 participants in three cohorts; 75 for visceral fat; 736 centenarians | mtDNA m.1382A>C genotype (K14Q MOTS-c) | Higher T2D prevalence in male carriers, strongest with low physical activity; higher visceral fat in male carriers (P < 0.05); no association with exceptional longevity |
Effects reported in the studies
- Insulin sensitivity and glucose handling (mice). Seven days of treatment raised the clamp glucose infusion rate by about 30 % in high-fat-fed mice and restored insulin-stimulated glucose uptake in 12-month-old soleus muscle to levels comparable to young mice1; 21 days of wild-type MOTS-c improved glucose tolerance in high-fat-fed male but not female mice4.
- Diet-induced obesity (mice). Weight gain over 8 weeks of high-fat diet was prevented with identical caloric intake, with lower insulin levels and less hepatic lipid1; reduced weight and fat mass were replicated in male but not female CD-1 mice over 21 days4.
- Physical performance and age-related decline (mice). Old (22-month) mice ran 2.0-fold longer and 2.16-fold farther after 2 weeks of treatment, and 17 % reached the sprint stage versus none of the controls; late-life intermittent treatment improved grip strength (P = 0.000078), stride length and walking capacity at >30 months, while lifespan was not significantly extended (P = 0.23)2.
- Cardiac function under exercise training (rats). Combined with treadmill training, MOTS-c raised myocardial mechanical efficiency from 31 % (exercise alone) to 66 % and the preload-recruitable stroke work slope from 71 to 103, whereas ejection fraction (72.6 % vs. 71.6 %) was not further changed; stroke work and cardiac output were lower than with exercise alone3.
- Bone loss after ovariectomy (mice). Twelve weeks of treatment significantly alleviated micro-CT-measured bone loss and inhibited RANKL-driven osteoclast differentiation, partly dependent on AMPK7.
- Endogenous MOTS-c in humans (observational). Acute cycling raised muscle MOTS-c 11.9-fold and plasma 1.6-fold in 10 young men2; lipid infusion raised plasma MOTS-c to 232-349 % of basal, which insulin blunted5; patients with coronary endothelial dysfunction had lower circulating MOTS-c (P = 0.007, n = 40)6; male carriers of the K14Q variant had higher type 2 diabetes prevalence in a 27,527-person meta-analysis4.
Adverse effects and tolerability reported
- No adverse events or toxicity reported in rodent studies. Mouse and rat studies up to lifelong follow-up describe no mortality, toxicity or histological adverse findings; formal toxicology endpoints were not part of any study design1,2,3,4,7.
- Reduced food intake. Old mice on late-life intermittent treatment ate significantly less in total (P = 0.00005)2; modest reductions in food intake and body weight were also seen after 4 days in normal-diet mice1.
- Sex-dependent response. Female high-fat-fed mice showed no change in body weight, fat mass or glucose tolerance with MOTS-c, in contrast to males4; the other rodent efficacy data come from male animals1,2,3.
- Suppression of mitochondrial respiration and antifolate-like mechanism. In vitro, MOTS-c reduced basal oxygen consumption under high glucose uptake, via folate-cycle inhibition and AICAR accumulation, a profile the authors compare to methotrexate1.
- Pro-inflammatory secretion in senescent cells (literature safety note). A review (Mendelsohn and Larrick 2018, Rejuvenation Res, PMID 30058454) summarises a report that MOTS-c and humanin exacerbate the senescence-associated secretory phenotype (IL-6, IL-1beta, IL-8, IL-10, TNF-alpha) in senescent cells in vitro; in contrast, MOTS-c reduced circulating IL-6 and TNF-alpha in mice1.
- Circulating MOTS-c as a stress marker rather than a benefit marker (human). In 125 Chinese adults without diabetes, plasma MOTS-c was elevated in metabolic syndrome (n = 26) and associated with waist circumference, liver fat and liver-damage markers (Sequeira et al. 2021, PMID 34419510); lipid infusion acutely raised it5. Elevated endogenous levels therefore do not indicate a favourable state.
- No direct vasoactive effect. MOTS-c did not change tone of isolated rat aortic rings or renal-artery-stenosis mouse vessels in organ chambers6.
Limitations of the evidence. Nearly all efficacy data on exogenous MOTS-c come from male rodents, and the two largest mouse programmes1,2 plus the variant study4 originate from a single group with declared financial ties to CohBar, Inc.; independent replication with quantitative endpoints is limited to smaller studies3,7. Human evidence is observational and concerns endogenous peptide levels, which rise with exercise but also with lipid load, liver fat and metabolic syndrome, so circulating MOTS-c cannot be read as a marker of benefit. No peer-reviewed human study of administered MOTS-c, and no formal toxicology, was found in PubMed; the lack of effect in female mice4 and the in vitro reports of SASP amplification and suppressed oxygen consumption remain unresolved. Several abstracts report significance without effect sizes1,7, which limits quantitative comparison.
References
- Lee C, Zeng J, Drew BG, Sallam T, Martin-Montalvo A, Wan J, Kim SJ, Mehta H, Hevener AL, de Cabo R, Cohen P (2015). The mitochondrial-derived peptide MOTS-c promotes metabolic homeostasis and reduces obesity and insulin resistance. Cell Metabolism. PMID 25738459 DOI
- Reynolds JC, Lai RW, Woodhead JST, Joly JH, Mitchell CJ, Cameron-Smith D, Lu R, Cohen P, Graham NA, Benayoun BA, Merry TL, Lee C (2021). MOTS-c is an exercise-induced mitochondrial-encoded regulator of age-dependent physical decline and muscle homeostasis. Nature Communications. PMID 33473109 DOI human study
- Yuan J, Wang M, Pan Y, Liang M, Fu Y, Duan Y, Tang M, Laher I, Li S (2021). The mitochondrial signaling peptide MOTS-c improves myocardial performance during exercise training in rats. Scientific Reports. PMID 34635713 DOI
- Zempo H, Kim SJ, Fuku N, Nishida Y, Higaki Y, Wan J, Yen K, Miller B, Vicinanza R, Miyamoto-Mikami E, Kumagai H, Naito H, Xiao J, Mehta HH, Lee C, Hara M, Patel YM, Setiawan VW, Moore TM, Hevener AL, Sutoh Y, Shimizu A, Kojima K, Kinoshita K, Arai Y, Hirose N, Maeda S, Tanaka K, Cohen P (2021). A pro-diabetogenic mtDNA polymorphism in the mitochondrial-derived peptide, MOTS-c. Aging (Albany NY). PMID 33468709 DOI human study
- Ramanjaneya M, Jerobin J, Bettahi I, Bensila M, Aye M, Siveen KS, Sathyapalan T, Skarulis M, Abou-Samra AB, Atkin SL (2019). Lipids and insulin regulate mitochondrial-derived peptide (MOTS-c) in PCOS and healthy subjects. Clinical Endocrinology (Oxford). PMID 31066084 DOI human study
- Qin Q, Delrio S, Wan J, Jay Widmer R, Cohen P, Lerman LO, Lerman A (2018). Downregulation of circulating MOTS-c levels in patients with coronary endothelial dysfunction. International Journal of Cardiology. PMID 29242099 DOI human study
- Ming W, Lu G, Xin S, Huanyu L, Yinghao J, Xiaoying L, Chengming X, Banjun R, Li W, Zifan L (2016). Mitochondria related peptide MOTS-c suppresses ovariectomy-induced bone loss via AMPK activation. Biochemical and Biophysical Research Communications. PMID 27237975 DOI
This section summarises findings published in the cited peer-reviewed literature for informational purposes. It is not a claim of efficacy or safety, contains no dosing or administration information by design, and does not constitute medical, veterinary or scientific advice. Results in cell cultures or animal models do not predict effects in humans.